Showing posts with label encephalization. Show all posts

Monday, July 30, 2012

That [obstetrical dilemma] really tied the [human evolution] together. Part 1.

Some impressive colleagues and I* are about to have a paper published that pulls the rug out from under a classic paleoanthropological hypothesis/theory.

Scratch that. If we're gonna do this Lebowski theme right, I just have to say that our paper will have “micturated upon” an old beloved rug, I mean story.

Trust me. Our research did not come from a “shut the [bleep] up, Donny” dismissive sort of place nor did it come from a “the bums will always lose” holier-than-thou sort of place. Nothing like that.

It came from honest to goodness seeking to understand, man.

Here's the old beloved story:

The obstetrical dilemma (OD) hypothesis = Simultaneous selection for big-brained (or simply big) babies and bipedal locomotion caused a dilemma because while babies must be large, birth canals must remain small. The consequences of this dilemma, which are often called “solutions” and “tradeoffs,” include (1) difficult and dangerous childbirth with universal assistance due to the tight fit, (2) relatively underdeveloped, helpless, often termed “secondarily altricial” neonates compared to all other primates which are precocial, and (3) compromised or sub-optimal female locomotion, since (4) selection has favored sexual dimorphism in the human pelvis with females having not just relatively wider but absolutely wider dimensions of the birth canal.

Notice how--like the way that a nice oriental rug spiffs up a dumpy Los Angeles living room--the OD skillfully ties together many unique or fascinating phenomena in human evolution, such as human bipedalism, human encephalization, hellish human childbirth, helpless (i.e. hellish?) human babies, male-biased human athletic ability, and broad ladies' hips.

And we haven't proven this story wrong. But we have thrown some serious doubt on it, demonstrating how little of it holds up to current evidence.

“This is our concern, Dude.”

Way back in grad school, my wise advisor Alan Walker gave me a copy of Adolf Portmann's A Zoologist Looks at Humankind in which he argues against a pelvic constraint on human gestation and fetal growth (the OD). So that primed me to carry some doubt in this OD world.

Then later, in 2007, I was post-doc-ing with Nina Jablonski and immersed in the mammalian life history, energetic, and encephalization literature. It occurred to me that, Oh goodie! I’ll find out how selection could have shortened our gestation as we became encephalized but as selection also maintained our small birth canals for bipedalism.

And not only did I strike out all around. But, I mean, the mammalian life history literature looks as if there’s absolutely nothing constrained about human gestation length or the timing of birth. If anything it looks like we’re weirder in the other extreme… having slightly longer gestations than other primates and having relatively big babies. Leading up to birth we’re actually suped-up primates, not limited ones. That we're not particularly different in these terms, and definitely not limited, has all been known for decades. I was late to the party.

When you look at Bob Martin's work, and others' like it (below), you see that the size of the mammalian mother predicts the length of gestation and the size of the offspring.


Manger, PR. 2006. An examination of cetacean brain structure with a novel hypothesis correlating thermogensis to the evolution of a big brain. Biol. Rev. 81: 293–338. "Fig. 17. Allometric plot of the relationship between neonatal (Mbirth) and adult body mass (Mb) in three orders of eutherian mammals. The data used in this plot are derived from that given in Nowack (1999)."


These predictions hold even when you look across mammals that have single births or litters and note how this includes encephalized mammals, like whales, that don't even have bony birth canals!


Sacher GA, Staffeldt EF (1974) Relation of gestation time to brain weight for placental mammals: implications for the theory of vertebrate growth. Am Nat 18(963): 593-615....Using an equation that takes into account neonatal brain weight, litter size, and “brain size advancement” (neonatal brain weight ∕adult brain weight),they predicted the gestation length for species of animals with known gestation length. These few variables, which exclude any pelvic dimensions, were successful at predicting gestation length in the vast majority of species in their study, including humans and the cetaceans which lack constricting bony birth canals.


It seems so obvious that there's an energetic limit to what a pregnant mammal mother can do. And it seems so not obvious that humans are exceptional as the OD would have it. And this perspective was strengthened after I read Peter Ellison's book On Fertile Ground: A Natural History of Human Reproduction in my spare time in the field one summer, fitting in a few pages after each hot day of Proconsul hunting, after retiring each night in my canvas tent on Rusinga Island.


“This [hypothesis] will not stand, man.”

So with all this research out there showing how birth seems to be limited primarily by maternal metabolism, why this notion that we’re compromised by our pelves? Why this notion that we could or should keep babies in our wombs longer if it wasn't for bipedalism keeping our birth canals too small for gestating any longer, for growing bigger babies?

After all, there was Anna Warrener (now at Harvard) presenting her dissertation research at our annual conference showing how wide hips aren't so bad for locomotion. And she cited other papers with similar results!

So why hadn't the OD been reevaluated yet given all this stuff. I wasn’t sure. And to be honest, I thought it was so obvious, this disconnect, this weakness of the obstetrical dilemma hypothesis that after I completed my first draft of the manuscript in 2008, I decided not to do anything with it. It was so obvious, to me, that it became so absolutely ridiculously pointless to write about it. But once I mustered up the gumption to send the manuscript out to several close friends (like Ken and Anne!) for a read and none of those clever folks said it was ridiculous, that’s when I felt some encouragement. It wasn’t ridiculous, it made sense. I just happened to be the first person that my friends had known to put it together.

Or so I thought.

Here I was ready to put this idea out there and then one of my readers, Jeff Kurland, a brilliant and beloved professor from my grad school days at Penn State mentioned, “I'm pretty sure Terry Deacon presented this same thing at the AAPAs back in the 1980s or ‘90s.”

This is when your heart sinks because you just went to all that trouble only to find out that someone already beat you to it. Again, I went back to thinking that my ideas must be so obvious to everyone in the field now. But no searching came up with any Deacon pubs on the topic so I wrote to him directly and he confirmed that he hadn't published it, but he shared the manuscript that he'd stopped working on long ago. It fit with mine in many ways--this doubt of the certainty that the bipedal pelvis is limiting further gestation length and fetal growth--and since he'd presented it publicly, I asked if he'd like to be on the paper and he did. This is when your heart soars because someone so clever shares your thinking. This idea is not ridiculous! (Plus, even if he had published it already, my paper could have been a much updated contribution and still not pointless. Hopefully I would have understood that, or at least someone would have shaken some sense into me.)

“You’re out of your element, [Holly].”

Right around the same time as I was getting this nice feedback from colleagues and friends I spoke to another close colleague, Herman Pontzer, about it. He's known as the "energetics guy" among other things so I figured he was the perfect litmus. And it seemed fairly straight forward to him. Again, it's not ridiculous. Hooray! I wasn't crazy! Plus now I had this fully capable human being on board, ready to replace my stolen figures from other pubs, to make similar points but with updated data. And, even better, he could test this hypothesis about maternal energetics by plotting out the data from various data sources. All was falling into place.

"This is what happens when you [birth] a [baby] in the [pelvis]!" ... “A world of pain.”


As we were putting our story together, I joked to a brand new mother, "You know, there's no obstetrical dilemma." And got a sharp-tongued, Oh yes there is, honey. I just went through labor. Hell yes there is!

In future such discussions, I was always sure to add, "...it's all energetics. A mom gives birth when she does because she can't possibly give any more energy into growing that fetus." And some moms who hear that are like, Duh! I could have told you that! 

You cannot win. At least I could not. But it was still encouraging.

By this point, we (Anna, Herman, Terry and I) had joined forces with Peter Ellison and we submitted our paper to a major journal for review. And I'll be back with a little digest of that paper and some thoughts on it a bit later...

Update, Sept. 1, 2012: Here's the next post. 

****

*Feynman's "half-advanced and half-retarded potentials" describes us nicely, with me as the latter.

Thursday, May 10, 2012

We need another explanation for our big brains like we need a hole in the head


(source)
Something was definitely up, up top, once our bodies, down below, committed to walking and running upright.

It’s only after things got familiarly human in the locomotor anatomy--when we got long legs, non-grasping toes, and reconfigured butts--that brains started increasing beyond ape proportions.

For the first four or five million years of hominin evolution (from 7-2.5 million years ago) the story’s about bipedalism. For the last two and a half, it’s about encephalization. We've known this thanks to fossils for a while and genetic evidence is saying the same thing. It’s natural, then, for such a cerebral organism to wonder whether the two are connected.

As you hypothesize, you could go the technology route. Freed forelimbs, not necessary for locomotion, are free to be handy. O! the possibilities for hurling turds and building worlds! So that's one idea: Selection for a brainier hominin (both physically and cognitively) could occur only after the hands were habitually free to be freaky.

You could go the ecology route. Once our bodies committed to bipedalism our diet changed to include more meat, hominin body size increased, and geographic dispersal did too, no doubt aided by our more efficient bodies built for long distance travel. These characteristics, together, have been compared to those of scavenging and predatory carnivores. Regardless of how small or large a part meat played in our ancestors’ diets, there’s no denying that an ecological shift occurred in the early Pleistocene, with an increase in diet and habitat diversity, and that shift must have included new requirements of the brain.

Or, you could go the sociality route. As hominins relied more and more on cooperative foraging and parenting behaviors, etc, navigating social networks became key. Once complex speech and language arrived, then there would be new demands on the brain as well.

These pressures, requirements, demands, however you want to think of them, could be working in concert and at different times (e.g. technology plus socializing) over deep, geologic time and many many hominin generations. By "working," I mean contributing to the more-or-less sustained differential reproductive success of hominins with slightly larger brains. And because it’s the way that the fossil and archaeological records reveal behaviors over time, I tend to think of these three categories (technology, ecology, sociality) as describing the last 2.5 million years in the order I listed them. Technology was strongest earliest (starting with the Oldowan stone tools by 2.6 mya), and persisted. An ecological shift came along with that technological shift and then persisted. And of course social complexity came along with the technological and ecological shifts and then persisted.

These are some of the most mainstream hypotheses for encephalization (1) and they're implicitly or explicitly predicated on the prior evolution of bipedalism.

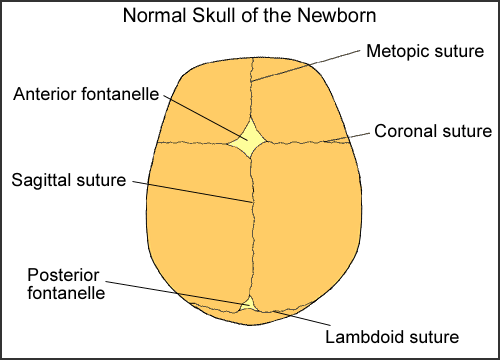
But now there's a new tie between big brains and walking upright--offered up in a  new paper just out in PNAS--and it's based in the human-, not ape-, like tendency to fuse the metopic suture later in life, to delay the close of what starts as a hole in the top of a baby's head known as its anterior fontanelle. The authors suggest that we need this hole in our head to exit our mother's bipedally-adapted birth canal safely and we also, as they suggest, need it to grow up to be an encephalized creature.

According to the authors, the "Taung child", an Australopithecus africanus kid (a member of a well-known bipedal hominin lineage) had an unfused metopic suture, left as an imprint on the fossil brain endocast.

Raymond Dart with the Taung child fossil.  http://en.wikipedia.org/wiki/File:Raymond_Dart_with_Taung.jpg 
Seven other australopith and Homo fossils are also described in the paper as having unfused metopic sutures. You might too! The odds are small, but since you started with a hole in your head as a baby, you could still be walking around with it unzipped.


To any chimps reading this, your metopic suture most likely closed just after birth and before your first deciduous molar erupted. But for 90% of humans (as reported in the paper), the suture closes later, after the eruption of the first deciduous molar. There’s a much slower fusion rate in humans than in chimpanzees.

However, to interpret the Taung child’s anatomy, things get a bit dicey, like things just love to get with hominin fossils. So often they can go either way: chimpy or humany.

Check out the figures below. A is for Pan troglodytes (common chimps) and B is for Homo sapiens. Those are frequencies of metopic suture fusion per dental age group. By listing them this way, instead of by chronological age, we're able to compare between two species that grow at different rates but share the same pattern of dental eruption. Chimpanzees grow up faster than us and experience earlier metopic suture fusion than us. Flipped around, humans grow up slower than chimps and experience delayed fusion of this suture compared to them. The Taung baby's dental age category is starred (*) at the "M1" stage in A and B. (The Taung child died at around 3.8 years of age, when its first permanent molar, M1, was erupted.)
Because it's more likely you'll find a human at that age (*) with an unfused metopic suture than a chimp, the researchers leaned toward calling the Taung child's state human-like, rather than ape-like. They backed that assertion up by listing seven other late Pliocene-early Pleiostocene hominins with unfused metopic sutures... it's a trend in the hominin lineage that begins with some australopiths, like the Taung child, they say.

"The presence of a still patent fontanelle and of a partially fused [metopic suture] in the Taung child, and the incidence of unfused [metopic sutures] in five adult and two other younger Australopithecus/ early Homo specimens is thus taken as evidence that a human-like pattern of late [metopic suture] fusion was already present in mid-to-late Pliocene gracile hominins."

Okay. Intriguing! But now we must explain!

[This is the part where, if you listen very carefully, you can hear the collective curmudgeonly groans from within and beyond the walls of paleoanthropology.]

Enter the new hypothesis for encephalization based on the late fusion of metopic sutures. The authors nod to two papers that offer "adaptively neutral" explanations for late metopic suture fusion but argue that the fossil evidence combined with the differences observed in chimps and humans beg for an adaptive explanation. (This tack is unsurprising given how paleoanthropology generally operates.)

The authors offer us three adaptive hypotheses to explain late metopic suture fusion:

1. Reorganization and expansion of the frontal neocortex (explains late metopic suture fusion)
Something about the changing and enlarging frontal cortex required changes to the cranial bones, how they form, grow, and fuse.

2. The difficulty of giving birth to large-headed neonates through birth canals that were reconfigured for bipedalism, the “obstetrical dilemma” (explains late metopic suture fusion)

The squishy neonatal head, thanks to the fontanelle,  "probably occurred in conjunction with refining the ability to walk on two legs," Falk (the lead author) said to the media. "The ability to walk upright caused an obstetric dilemma. Childbirth became more difficult because the shape of the birth canal became constricted while the size of the brain increased. The persistent metopic suture contributes to an evolutionary solution to this dilemma."

The trouble with this hypothesis as applied here is, although we know modern humans have a tight fit at birth now, there's little evidence for a tight fit between neonate and birth canal during australopith times.

And you can't help but wonder whether a squishy head was, or still is, required for successful birth. Do children suffering from craniosynostosis require a c-section to be born? Also, since the metopic suture fuses after chimpanzee birth, are we certain they aren't squishing their brains as they exit their relatively roomy birth canals? These questions may sound silly, but they're illustrating the built-in assumptions of the paper (or my ignorance about squishiness of baby heads).

The squishy head may be helpful during childbirth, but if it's occuring as early as australopith times, an adaptive explanation as a "solution" to an obstetrical dilemma is hard to swallow. That is unless DeSilva's estimates cited by the authors-- that australopiths had large neonates and tight fits at birth--are correct.

3. High early postnatal brain growth rates (explains late metopic suture fusion)
We know that humans have high rates of postnatal brain growth and this is what a lot of the news media picked up on: Your baby's head has gaps between the bones so the brain can grow like crazy after it's born to the gargantuan size of an adult human brain. As established in hypothesis #2, the need for the fontanelles in the first place is the crunch at birth thanks to the obstetrical dilemma, implying that without the pressure to be born small enough to escape the bipedal birth canal, we'd grow larger fetal brains in the womb.

So with this new paper we're presented with something even more fundamental than the notion that bipedalism as a necessary precursor for technological, ecological and social selection pressures for encephalization (as covered above): The tight fit at birth, caused by antagonistic selection for bipedal pelvic anatomy and large neonatal brains, created the selection pressure for a squishy neonatal head (which is facilitated by the fontanelles) and because of that roomy cranium, postnatal growth rates were able to ramp up in selective environments that favored encephalization.

So I'm left wondering, Do we need a hole in our head to be born successfully? Do we need a hole in our head to be encephalized? If the answer to both of those is yes, then what is a hole in the head doing in a hominin genus that may not have had much difficulty with childbirth and was hardly (if at all) encephalized? And, given the overlapping chimp and human fusion patterns, how can we be sure this feature on Taung is humany and not chimpy?

And, further, you can't (or at least I can't) help but wonder if there's a biomechanical/functional explanation for late metopic suture fusion, given how feeding behaviors and masticatory muscles put stress on the cranium. The skulls of australopiths and other hominins experienced stresses differently than chimpanzees. These differences may have begun as early as the nursing stage. Could this have anything to do with delayed fusion of the sutures? (here's just one study I found that addresses these kinds of questions)

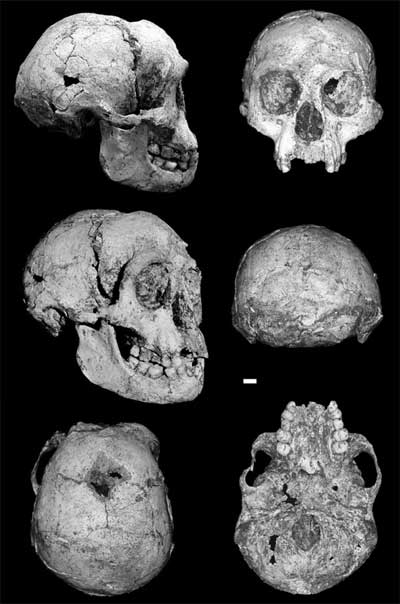
And finally, it's hard not to link Falk (the lead author) to her research on Homo floresiensis. The hobbit (LB 1) looks like it has a fontanelle, something the disease-hypothesis folks point out is consistent with their perspective, and that’s one reason why I assumed these authors are onto this topic.

But LB 1 is conspicuously absent from the laundry list of hominin fossils in the supplementary section. Either they're saving what they've got on metopic suture and fontanelle anatomy in H. floresiensis for an upcoming paper or they just didn't think it was worthwhile to include this specimen. After all,  the latest paper on hobbit anatomy claims that the hobbit's "fontanelle" isn't real. Peter Brown writes, "direct examination of the asymmetrical hole in the posterior frontal of LB1, supported by CT scans, clearly indicates that this is the result of post-mortem excavation damage and is definitely not an unfused anterior fontanelle." (2)

Good thing, because if the hole in LB 1's cranium is of biological and not of taphonomic origin, then who knows how anybody'd explain its adaptive significance in such a tiny-brained hominin.

But, going way back to Taung and the australopiths: They were, after all, bipedal and the big brain train had to pull out at some point!

And, stay tuned. I got a tip from one of the authors about a paper coming out soon that demonstrates how weak the obstetrical dilemma hypothesis is, for explaining fetal size and growth, given the current evidence and given what we know about maternal metabolism.

Notes
(1) Of course, these hypotheses don’t represent all of paleoanthropology. I just intended to cover the major bases. And you need to consider what many paleoanthropologists assume which is that brain tissue is expensive so something extraordinary must have kept up selection on its increasing size for the last 2.5 million years. The assumption is that if brains were cheap, everyone would have big ones, but I don’t buy that. I think it's clear that other species aren’t encephalized because they don’t have to be. They do just fine without big brains. We have a rather warped perspective on selection for encephalization, thanks to our presentism and our big brains.
(2) Thanks to K. Baab for the tip.